

We investigate the mechanisms that prevent mutagenesis in the germline. 🧪🧬👨🔬 @MRC_LMB
Joined April 2018
- Tweets38
- Following166
- Followers135
- Likes49


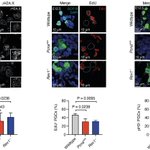


Most surprisingly, upon loss of TLS there is a genome-wide failure of DNA demethylation: a critical step in the process of epigenetic reprogramming during germ cell development, as well as a failure to engage the germ cell transcriptional network.
In embryonic germ cells loss of the TLS pathway results in increased DNA damage, activation of cell cycle arrest, and the induction of apoptosis - leading to an over 99% reduction in embryonic germ cells and ultimately leading to complete sterility of adults.
We discovered that TLS factors are required for the development of germ cells in the embryonic stages in both human and mouse. In contrast, TLS was dispensable for the maintenance of somatic tissues.
Delighted to share our most recent paper explaining why DNA Translesion Synthesis (TLS) is required for fertility. Huge amount of work from @Pranay_Shahh and a great collaboration with @ReikLab at Altos Labs, @HGLeitch and the Garaycoechea Lab @_Hubrecht Institute (link below)
In summary, we find that the Fanconi anemia crosslink repair pathway acts as a ‘fail-safe’ to prevent L1 retrotransposition when other canonical restriction mechanisms are absent. 9/9
Finally, we show that not only embryonic but also maternal factors are important to suppress L1 retrotransposition at the earliest stages of development 8/n
We find that testes, but more specifically, sperm derived from Fanconi-deficient mice accumulate high levels of L1 retrotransposition compared to somatic tissues 7/n
Organisms restrict L1 retrotransposition mainly by transcriptional silencing. However, during embryonic and germline development this mechanism is attenuated 6/n
To study if this holds in vivo, we employ the previously characterised SN1 L1 reporter and find that Fanconi-deficient mice accumulate high levels of L1 integrations in multiple tissues 5/n
By purifying the crosslink incision complex (SLX4-XPF-ERCC1), we demonstrate that it can cleave putative intermediates of L1 retrotransposition and therefore abort new integrations 4/n
As many factors involved in FA repair restrict L1 retrotransposition, we generate double knockouts and find that they act in a common pathway to limit L1 integrations 3/n
We first confirm that many DNA repair factors regulate L1 retrotransposition in human cells, either by suppressing or promoting new integrations 2/n
Very excited to share our latest work nature.com/articles/s41594-0… published in @NatureSMB ! We find that the Fanconi Anemia DNA crosslink repair pathway restricts L1 retrotransposition during mouse development 🐭🧬 🧵 1/n

In all, TLS components are dispensable in the somatic lineages but essential in the germline. PGCs lacking TLS factors fail to express germline genes or perform global DNA demethylation showing a developmental block, explaining infertility of TLS-deficient organisms
8/9

Molecular characterisation of mutant day 12.5 PGCs shows a failure of global DNA demethylation. The level of methylation is more similar to epiblast cells than PGCs. The germline transcriptional programme is also corrupted with mutant PGCs failing to engage germline genes 7/9

In the absence of REV1 and upon mutation of PCNA K164, PGCs display higher burdens of DNA damage, perturbed cell cycle dynamics and reduced proliferation 6/9

However, PCNA K164 modification is dispensable for maintaining all somatic lineages studied revealing a striking dichotomy between the germline and soma 5/9

